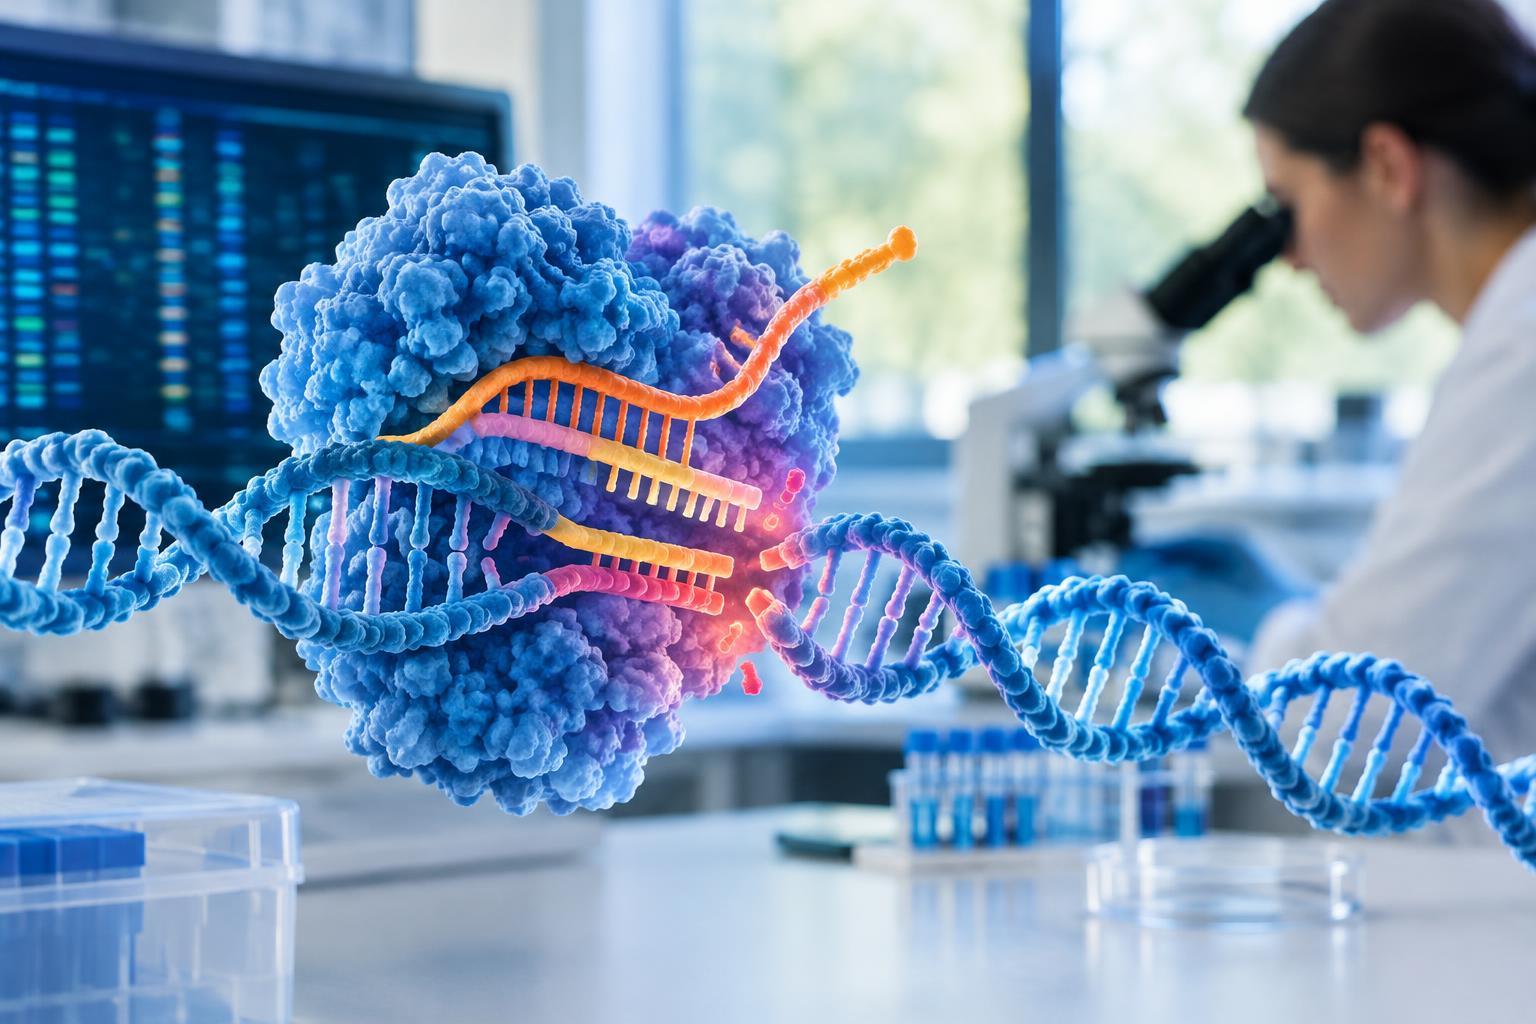
1. CRISPR Is a Targeting System, Not a Genetic Word Processor
CRISPR gene editing grew out of defense systems that bacteria and archaea use against invading genetic material. Researchers adapted components of these systems into tools that recognize selected DNA sequences. The best-known example pairs a guide RNA with the Cas9 protein, an enzyme that can cut DNA.
The guide RNA contains a targeting sequence designed to pair with a stretch of DNA. Cas9 also requires a nearby short DNA motif called a PAM. Different Cas proteins recognize different PAMs, which helps determine where each tool can act. Once Cas9 encounters a suitable PAM, it can check the neighboring DNA for a match to the guide.
This targeting is powerful, but it is not equivalent to clicking a word and replacing it. DNA is packaged inside cells, sequence recognition is imperfect, and the cell's response often determines the eventual edit.
2. Finding and Cutting the DNA Target
In a conventional Cas9 experiment, researchers select a target sequence and design a corresponding guide. They then deliver the editing components into cells. These may arrive as a preassembled protein–RNA complex or as genetic instructions that the cell uses to produce the components.
When enough matching occurs between the guide and target DNA, active Cas9 cuts both DNA strands near the target site. This creates a double-strand break. The cut itself does not specify the final genetic outcome: it mainly creates a problem that the cell must repair.
Target accessibility also matters. DNA wrapped around proteins or packed into less accessible chromatin may be harder to reach. Two guides that look similarly promising from their sequences can therefore perform differently in actual cells.
3. Cellular Repair Determines Much of the Result
One common repair route is end joining, in which the cell reconnects the broken DNA ends. Classical nonhomologous end joining can restore the original sequence, but processing of the ends can also produce small insertions or deletions. Other end-joining pathways may contribute additional changes. Researchers often exploit these outcomes to disrupt a gene.
Disruption is not guaranteed. An insertion or deletion within a protein-coding region may shift the reading frame, changing how the sequence is translated. Other edits preserve the frame, and some leave enough function intact for the gene to remain active. Cutting a gene and successfully disabling it are therefore different experimental claims.
For a planned sequence change, researchers may supply a DNA repair template carrying the desired sequence alongside matching regions. Through homology-directed repair, the cell can copy information from that template into the damaged site. However, this pathway competes with other repair processes and is generally more accessible during particular stages of the cell cycle. Its efficiency varies substantially by cell type and experimental conditions, especially in cells that do not divide.
4. Not Every CRISPR Editor Makes a Double-Strand Break
Base editors combine a modified targeting protein with an enzyme that chemically changes certain DNA bases. Common versions support particular classes of single-letter substitutions without deliberately cutting both DNA strands. Their reach is limited by targeting requirements and a local editing window, and they may change additional susceptible bases within that window.
Prime editors combine a modified Cas protein with a reverse transcriptase and a specialized guide RNA that carries the proposed edit. They can introduce a broader range of substitutions and some small insertions or deletions without a conventional double-strand break. Neither approach removes all uncertainty: efficiency, unwanted products, and delivery remain important constraints.
5. Precision Has Several Biological Limits
Off-target editing occurs when an editor acts at an unintended location, often one resembling the intended target. Guide design and engineered proteins can reduce this risk, but the absence of changes at a few predicted sites does not establish that none occurred elsewhere.
Unwanted outcomes can also occur at the correct target. Double-strand breaks may produce larger deletions or rearrangements rather than only the expected small changes. A cell population can contain a mixture of unedited cells, correctly edited cells, and cells carrying other outcomes. Different DNA copies within one cell may also be edited differently.
Delivery adds another limitation. Components must reach the relevant cells, enter them, and access their DNA while remaining sufficiently active. Tissue barriers, cell stress, and immune responses can complicate that process. Finally, many traits depend on multiple genes and environmental influences, so a precise DNA change does not necessarily produce a simple or predictable biological effect.
6. How to Interpret a CRISPR Result
A convincing editing result requires more than evidence that Cas9 reached its target. Researchers need to establish which sequences changed, how frequently the intended outcome occurred, and whether relevant unintended outcomes appeared. They must also test whether the edit produced the expected functional effect.
When reading about CRISPR, distinguish targeting accuracy, editing efficiency, and biological benefit. These answer different questions. CRISPR makes DNA experimentally addressable with remarkable flexibility, but cellular repair and biological context still shape what happens after the target is found.


